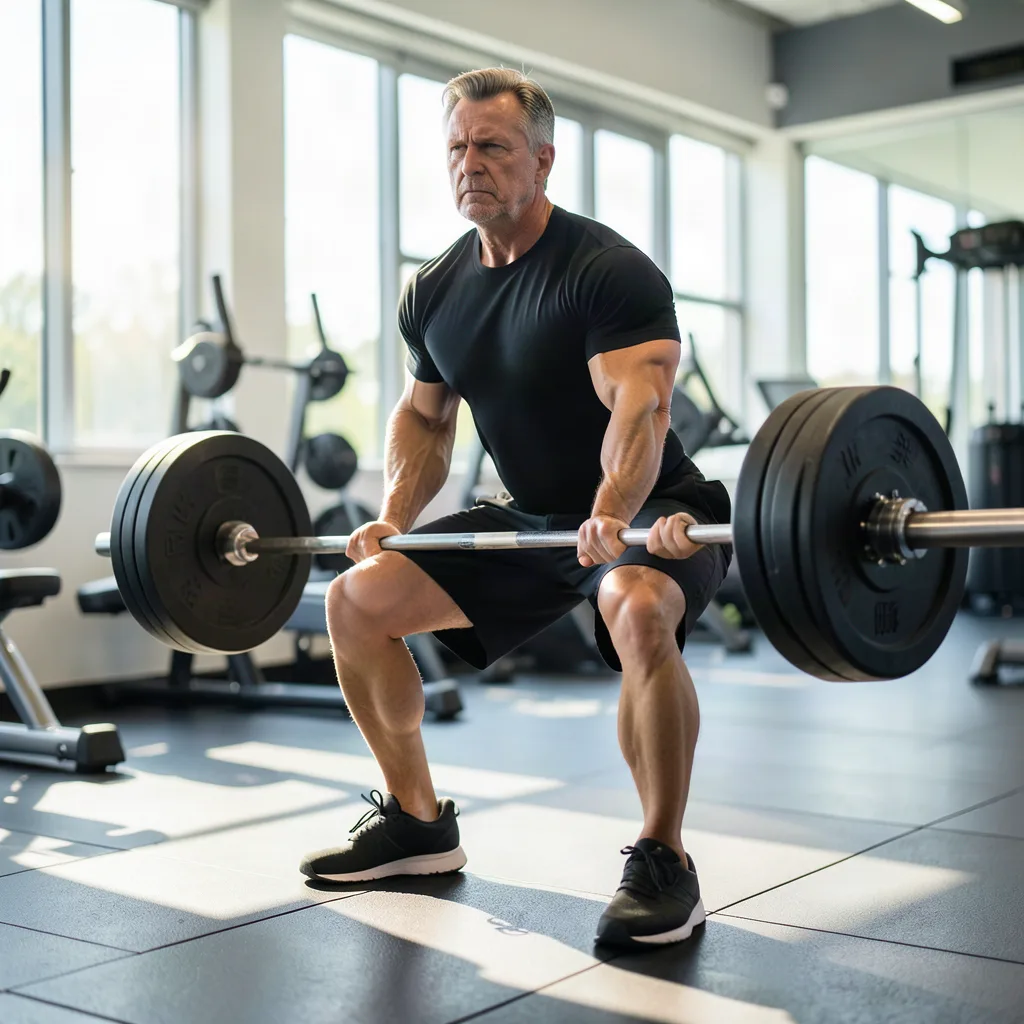
Leg day often gets a reputation for being the most dreaded workout of the week, but emerging research shows that training the lower body does far more than build strong quads and glutes. Regularly challenging the largest muscle groups in the body triggers a cascade of hormonal, vascular, and neural signals that support cognitive function, memory, and mood. This article explores the science behind the leg‑brain connection and gives practical ways to make lower‑body training a cornerstone of lifelong brain health.
Key takeaways
- Compound movements like squats and deadlifts stimulate the release of brain-derived neurotrophic factor, which supports neuronal growth and health.
- Lower-body training increases cerebral blood flow and oxygenation, helping the brain clear metabolic waste products and improve synaptic plasticity.
- Regular leg workouts are linked to a lower risk of cognitive impairment and help maintain executive function and processing speed as you age.
- Combining physical leg exercises with mental tasks, such as word recall, can further enhance neuroplasticity and prefrontal cortex activity.
The Physiology of Leg Training and the Brain
When you perform compound movements such as squats, deadlifts, or lunges, you recruit a massive amount of muscle fibers across the hips, thighs, and calves. This recruitment demands a high level of motor unit activation, which sends strong afferent signals to the central nervous system. The brain responds by up‑regulating neurotransmitter systems that are involved in attention, learning, and mood regulation. Studies using functional MRI have shown increased activation in the prefrontal cortex and hippocampus after a single bout of heavy lower‑body resistance exercise.
Because the legs contain the largest muscle mass in the human body, the metabolic cost of leg training is disproportionately high. This creates a systemic demand for oxygen and nutrients that stimulates cardiovascular adaptations. Improved cerebral perfusion follows, delivering more glucose and oxygen to neurons during both exercise and rest. The net effect is a brain that receives a richer supply of the fuel it needs for synaptic plasticity.
Hormonal Surge: Growth Factors and Neurotrophins
Heavy leg workouts provoke a sharp rise in anabolic hormones such as testosterone, growth hormone, and insulin‑like growth factor‑1 (IGF‑1). These hormones cross the blood‑brain barrier and bind to receptors in regions responsible for memory consolidation. IGF‑1, in particular, has been shown to promote neurogenesis in the dentate gyrus of the hippocampus, a process essential for forming new memories.
In addition to classic anabolic hormones, resistance training stimulates the release of brain‑derived neurotrophic factor (BDNF). BDNF acts like fertilizer for neurons, supporting dendritic branching and long‑term potentiation. Research indicates that lower‑body training performed at moderate to high intensity produces a larger BDNF response than comparable upper‑body sessions, likely because of the greater overall muscle mass engaged.
Blood Flow and the Blood‑Brain Barrier
During a set of heavy squats, cardiac output can increase by 30‑40 percent, and a significant portion of that extra flow is directed to the working muscles. The vascular shear stress generated by this surge triggers endothelial nitric oxide synthase, raising nitric oxide levels systemically. Nitric oxide is a potent vasodilator that also enhances the integrity of the blood‑brain barrier, reducing neuroinflammation and allowing beneficial circulating factors to reach neural tissue more efficiently.
Chronic leg training leads to structural remodeling of the cerebral vasculature, including increased capillary density in the motor cortex and hippocampus. This angiogenesis improves the brain’s ability to clear metabolic waste products such as beta‑amyloid, a protein implicated in Alzheimer’s disease. In practical terms, a consistent leg routine may serve as a non‑pharmacological strategy to maintain vascular brain health across the lifespan.
Muscle‑Brain Communication Through Myokines
Skeletal muscle is now recognized as an endocrine organ that secretes myokines—peptide hormones released during contraction. Interleukin‑6 (IL‑6), irisin, and cathepsin B are among the myokines that have documented effects on the central nervous system. IL‑6, for example, can cross the blood‑brain barrier and modulate hypothalamic pathways that regulate energy balance and mood.
Irisin, discovered in 2012, is upregulated by resistance exercise and has been shown to increase BDNF expression in the hippocampus. Cathepsin B, another exercise‑induced myokine, correlates with improved spatial memory in animal models. Because the lower limbs generate the greatest total myokine output due to their size, leg‑dominant workouts amplify this muscle‑to‑brain signaling pathway more effectively than isolated upper‑body training.
Strength Gains Translate to Cognitive Resilience
Longitudinal studies linking muscular strength to cognitive outcomes consistently find that lower‑body strength is a stronger predictor of executive function and processing speed than grip strength alone. One prospective cohort of older adults showed that participants in the highest quartile of leg press performance had a 40 percent lower risk of developing mild cognitive impairment over a ten‑year follow‑up.
The mechanism likely involves both the direct neurobiological effects described above and the functional independence that strong legs provide. Maintaining mobility enables continued participation in socially and cognitively stimulating activities—dance classes, hiking, group sports—which themselves protect brain health. Thus, leg strength creates a positive feedback loop: stronger legs → more activity → richer cognitive environment → preserved neural networks.
Designing an Effective Leg‑Focused Routine
To harness the brain‑boosting potential of leg training, aim for two to three dedicated sessions per week. Each session should include at least one multi‑joint compound movement (back squat, front squat, deadlift, or hip thrust) performed for three to five sets of five to eight repetitions at 70‑85 percent of one‑rep max. Complement the primary lift with accessory work such as Bulgarian split squats, Romanian deadlifts, and calf raises to address unilateral imbalances and tendon health.
Progressive overload is essential. Increase load, volume, or range of motion every one to two weeks while monitoring recovery markers such as resting heart rate variability and subjective fatigue. Incorporate tempo variations—slow eccentrics of three to four seconds—to maximize mechanical tension and myokine release without excessive joint stress.
Recovery, Sleep, and Neuroplasticity
The brain benefits of leg training are realized during recovery, not during the workout itself. Deep non‑REM sleep is when growth hormone peaks and BDNF consolidates synaptic changes made during the day. Prioritize seven to nine hours of quality sleep, and consider a short nap after an especially intense leg session if nighttime sleep is compromised.
Active recovery strategies—light cycling, mobility drills, contrast showers—enhance lymphatic clearance of metabolic byproducts and reduce systemic inflammation. Nutrition also plays a role: adequate protein (1.6‑2.2 g per kg body weight), omega‑3 fatty acids, and polyphenol‑rich foods support both muscle repair and neuronal membrane fluidity.
Integrating Leg Work Into a Busy Lifestyle
Time constraints are the most common barrier to consistent leg training. A practical solution is to adopt a “micro‑dosing” approach: perform a single heavy compound set (e.g., five‑rep back squat) at the start of each workout day, regardless of the primary focus. Over a week this accumulates to three to four high‑quality leg stimuli without requiring a full dedicated session.
For those with limited equipment, bodyweight variations such as pistol squat progressions, jump squats, and walking lunges can generate sufficient mechanical load when performed with controlled tempo and high effort. Resistance bands and a single kettlebell expand the exercise library dramatically. The key is consistency—any regular lower‑body stimulus is superior to sporadic maximal efforts.
Neuroimaging and Structural Brain Adaptations from Chronic Leg Training
Longitudinal magnetic resonance imaging studies reveal that adults who perform progressive lower‑body resistance training for six months or longer show measurable increases in hippocampal volume, particularly in the dentate gyrus where adult neurogenesis occurs. Diffusion tensor imaging further demonstrates enhanced fractional anisotropy in the corpus callosum and the superior longitudinal fasciculus, indicating improved white‑matter integrity that supports faster inter‑hemispheric communication. Functional MRI during resting state shows stronger connectivity within the default mode network and the frontoparietal control network, both of which are critical for working memory and executive planning. A dose‑response relationship emerges: participants who accumulate at least 120 minutes of heavy compound leg work per week exhibit the greatest volumetric gains, while those training once weekly show modest but statistically significant changes. Importantly, these structural adaptations correlate with performance on standardized neuropsychological batteries such as the Trail Making Test and the Rey Auditory Verbal Learning Test, providing a direct link between the mechanical stimulus of squats or deadlifts and measurable cognitive outcomes. Researchers hypothesize that the repeated surges in cerebral blood flow, BDNF, and IGF‑1 during each session create a permissive environment for synaptic remodeling, and that the mechanical loading itself may activate mechanosensitive pathways in astrocytes that further support vascular coupling. Practically, athletes and recreational lifters can track progress by scheduling an annual brain MRI or, more accessibly, by monitoring cognitive test scores every three months alongside strength metrics.
Timing and Circadian Alignment: When to Train Legs for Maximal Cognitive Gain
Circadian biology modulates the hormonal milieu that underlies the leg‑brain axis. Testosterone and growth hormone peak in the early morning, while cortisol rises sharply after awakening and declines throughout the day. Training the largest muscle groups during the morning window (approximately 07:00‑09:00) leverages the natural anabolic surge, amplifying the IGF‑1 and BDNF response without the catabolic interference of elevated evening cortisol. Conversely, evening sessions (18:00‑20:00) benefit from higher core temperature and greater neuromuscular efficiency, which can allow heavier loads and thus a larger mechanical signal. Emerging data from time‑of‑day experiments suggest that morning leg workouts produce a more pronounced acute improvement in attention and mood, whereas evening workouts yield greater gains in procedural memory consolidation during subsequent sleep. For shift workers or individuals with delayed chronotypes, aligning the primary leg session to the personal circadian peak—identified via wearable temperature or melatonin profiling—optimizes neurotrophic release. A practical schedule might involve a heavy compound lift (e.g., back squat 5 × 5 at 80 % 1RM) at the identified peak, followed by a lighter accessory circuit later in the day to maintain metabolic stimulus without overtaxing recovery. Consistent sleep‑wake timing, exposure to bright light within 30 minutes of waking, and avoidance of caffeine after 14:00 further stabilize the hormonal rhythms that make leg training a reliable cognitive enhancer.
Dual‑Task and Cognitive‑Motor Integration: Pairing Leg Work with Brain Challenges
Combining lower‑body resistance or plyometric movements with simultaneous cognitive tasks creates a synergistic environment for neuroplasticity. In laboratory settings, participants who performed walking lunges while completing an auditory n‑back task showed greater increases in prefrontal oxygenation (measured by functional near‑infrared spectroscopy) and larger post‑exercise BDNF spikes than those who performed either activity alone. The mechanism likely involves heightened attentional demand that forces the prefrontal cortex to allocate resources to both motor planning and working‑memory updating, thereby strengthening shared neural circuits. Practical implementations include: (1) performing a set of goblet squats while reciting a memorized list of words, (2) executing box step‑ups in rhythm with a metronome that randomly changes tempo, requiring rapid decision‑making, or (3) using a smartphone app that presents visual‑spatial puzzles during rest intervals of a leg‑press circuit. For older adults, a safe entry point is seated heel‑raise sequences paired with simple verbal fluency prompts (e.g., name as many animals as possible in 30 seconds). Progression can be achieved by increasing the cognitive load (higher n‑back level) or the mechanical load (adding external resistance) but not both simultaneously, to avoid excessive dual‑task cost that could compromise form. Research indicates that 8‑week dual‑task programs improve gait speed, balance confidence, and executive function scores more than single‑task training, making this approach valuable for fall prevention and cognitive preservation alike.
Sex‑Specific Responses and Hormonal Milieu in Leg‑Brain Signaling
Estrogen and progesterone modulate the expression of BDNF receptors and the sensitivity of the hypothalamic‑pituitary‑gonadal axis to resistance exercise. During the follicular phase, higher estradiol levels amplify the BDNF response to a given leg‑training stimulus, while the luteal phase’s elevated progesterone can blunt the acute testosterone surge but may enhance GABAergic tone, favoring recovery and sleep quality. Post‑menopausal women experience a marked decline in estrogen, which correlates with reduced hippocampal plasticity; however, consistent heavy leg training (2‑3 sessions per week at ≥75 % 1RM) has been shown to partially restore BDNF levels and improve verbal memory to values comparable with pre‑menopausal controls. In men, the larger absolute testosterone response to squats and deadlifts yields a more pronounced IGF‑1 elevation, yet the relative percent increase in BDNF is similar across sexes when training intensity is matched. Practical programming implications: women may benefit from scheduling the heaviest leg session during the early follicular window (days 3‑7) to capitalize on estrogen‑mediated neurotrophic potentiation, while incorporating lighter, higher‑volume accessory work in the luteal phase to support recovery. For both sexes, tracking menstrual cycle phase or using salivary hormone panels can individualize load progression, ensuring that the neuroendocrine environment remains favorable for brain‑derived adaptations.
Leg Training for Clinical Populations: Stroke, Parkinson’s, and Mild Cognitive Impairment
Rehabilitation guidelines increasingly incorporate progressive lower‑body resistance as a disease‑modifying intervention. In chronic stroke survivors, bilateral leg press training at 60‑70 % 1RM three times weekly for 12 weeks increased paretic‑side cortical excitability (measured by transcranial magnetic stimulation) and improved scores on the Montreal Cognitive Assessment. The bilateral nature of the exercise promotes inter‑hemispheric inhibition balance, a key factor in motor recovery and cognitive re‑engagement. For individuals with Parkinson’s disease, high‑velocity concentric leg extensions combined with cueing (auditory metronome) enhance dopaminergic transmission in the striatum, leading to measurable gains in set‑shifting tasks and reduced freezing of gait episodes. Mild cognitive impairment cohorts who added a twice‑weekly hip‑thrust protocol (3 × 8 at 75 % 1RM) to standard aerobic care showed a 15 % reduction in amyloid‑β plasma ratios and improved episodic memory after six months. Safety considerations include: monitoring blood pressure response during heavy eccentrics, using belt‑squat or sled‑push variations to unload the spine in osteoporotic patients, and employing real‑time heart‑rate variability feedback to avoid autonomic overload. Multidisciplinary teams should integrate neuropsychological testing at baseline, 3 months, and 6 months to quantify cognitive trajectories alongside strength metrics, allowing dose adjustments that maximize neuroprotective benefit while minimizing adverse events.
Monitoring and Quantifying the Leg‑Brain Axis with Wearable Technology
Advances in consumer‑grade sensors now enable real‑time tracking of the physiological mediators that link leg training to brain health. Heart‑rate variability (HRV) measured via chest strap or wrist photoplethysmography provides a proxy for autonomic balance; a sustained increase in the root‑mean‑square of successive differences (RMSSD) across training weeks correlates with higher BDNF concentrations in validation studies. Near‑infrared spectroscopy (NIRS) headbands placed over the prefrontal cortex capture task‑evoked oxygenation changes during and after squat sets, offering a direct window into cerebrovascular reactivity. Portable force plates embedded in smart insoles quantify ground‑reaction forces and rate of force development during lunges or jumps, allowing coaches to ensure that mechanical stimulus thresholds (≥2.5 × body weight peak force) are met for optimal myokine release. Some platforms integrate these streams into a single dashboard that flags when HRV drops >15 % from baseline, suggesting insufficient recovery and potential cortisol‑mediated neuroinflammation. Machine‑learning models trained on longitudinal datasets can predict individual cognitive‑performance trajectories (e.g., Stroop test improvement) from combined strength, HRV, and NIRS features, enabling personalized periodization. Practically, athletes can adopt a weekly “neuro‑check” session: a standardized 5‑rep back squat at 80 % 1RM while wearing the sensor suite, followed by a 2‑minute cognitive battery on a tablet. The resulting data inform whether to progress load, insert a deload week, or adjust sleep hygiene, turning subjective feeling into objective, brain‑centric decision making.
Nutrition, Supplementation, and Gut‑Brain Crosstalk to Amplify Leg‑Derived Neurotrophic Signals
The metabolic aftermath of heavy leg sessions creates a nutrient‑sensing environment that can be steered toward greater neuroplasticity. Consuming 30‑40 g of high‑quality protein (whey isolate or a blended plant source) within 30 minutes post‑exercise maximizes muscle‑protein synthesis and provides the amino‑acid precursors (especially leucine) required for central BDNF translation. Omega‑3 fatty acids (EPA + DHA 2‑3 g daily) incorporate into neuronal membranes, enhancing fluidity and facilitating TrkB receptor signaling downstream of BDNF. Polyphenol‑rich foods—blueberries, dark cocoa, green tea—activate the Nrf2 pathway, reducing oxidative stress that otherwise degrades activity‑dependent neurotrophins. Creatine monohydrate (5 g daily) has been shown to augment phosphocreatine resynthesis in both muscle and brain, improving performance on working‑memory tasks after resistance training. Dietary nitrate from beetroot juice (≈400 mg nitrate 2‑3 hours pre‑workout) boosts nitric‑oxide bioavailability, further supporting cerebral perfusion during the leg‑induced shear‑stress surge. Emerging evidence links gut microbiota composition to systemic BDNF levels; a diverse fiber intake (≥30 g/day from varied vegetables, legumes, and whole grains) promotes short‑chain fatty acid production (butyrate) that crosses the blood‑brain barrier and up‑regulates BDNF transcription. A sample day for a 80 kg lifter might include: pre‑workout beetroot shot + 20 g whey; intra‑workout 6 % carbohydrate‑electrolyte solution; post‑workout 40 g whey + 1 g creatine + 1 g EPA/DHA; lunch salmon, quinoa, roasted broccoli, mixed berries; snack Greek yogurt with walnuts; dinner chicken thigh, sweet potato, kale salad with olive oil; before bed 20 g casein + 500 mg magnesium glycinate. This nutritional framework ensures that the mechanical, hormonal, and vascular signals generated by leg training are met with the substrates needed for lasting cognitive enhancement.
Frequently Asked Questions
Does leg training improve memory in young adults as well as older adults?
Yes. Controlled trials with university students have shown that a single bout of heavy squats increases BDNF and improves performance on working‑memory tasks measured 30‑60 minutes post‑exercise. The magnitude of the effect scales with training status, but even novices experience measurable cognitive gains.
Can I replace leg day with high‑intensity interval training for brain benefits?
High‑intensity interval training (HIIT) that includes lower‑body movements such as sprinting or cycling can elicit similar hormonal and myokine responses. However, the mechanical loading of heavy resistance exercise uniquely stimulates osteogenic and tendon adaptations that support long‑term mobility, which indirectly sustains cognitive engagement. A combined approach—resistance leg work plus occasional HIIT—offers the most comprehensive benefit.
What if I have knee or hip issues that limit heavy squats?
Joint‑friendly alternatives include box squats to a comfortable depth, belt‑squats, hip thrusts, and sled pushes. These movements load the posterior chain and quadriceps while reducing compressive forces on the knee. Consulting a physical therapist for individualized programming ensures you still capture the systemic neurobiological stimulus without aggravating pathology.
How quickly can I expect to notice cognitive changes after starting leg training?
Acute improvements in attention and mood can appear after the first few sessions due to neurotransmitter and BDNF spikes. Structural brain changes such as increased hippocampal volume typically require months of consistent training, mirroring the timeline for measurable strength gains. Tracking subjective focus, sleep quality, and reaction‑time tests can provide early feedback.
Is there an upper limit where too much leg training harms brain health?
Excessive volume without adequate recovery can elevate chronic cortisol and systemic inflammation, which may impair neurogenesis and increase oxidative stress in the brain. Signs of overtraining include persistent fatigue, sleep disturbance, and declining performance. Periodizing training—alternating high‑intensity blocks with deload weeks—protects both muscular and neural adaptations.
Related posts:
 Perfect Your Glute Bridge
 This Full-Body Resistance Band Workout Will Transform Your Home Gym
 Understanding Gym Equipment
 Get Stronger with Charlee Atkins
 Sitting Too Much Might Lead to Memory Loss
 How to Change Your Fitness Routine to Avoid Plateau
 PHA Bodyweight Workout: Efficient Fitness Anywhere, Anytime
 Brain-Boosting Foods